


Likes
Comments
Share


@MrGoonai
Follow
02/03/25 Short facts:
- 58cm high
- Light is @80% but in a distance of 24 to 35cm - 600 to 740 ppfd
- VPD increased to 1.0 but I only do get it up to 0.9
- Defoliated again
---------------------------------------------------------------------------------
She has grown significantly again, becoming taller and producing more leaves. I had to defoliate her once more, but she has already regrown some leaves, so I'll probably have to defoliate her again this week.
I'm really impressed, she's doing so well!
Likes
93
Share


@OrganicNature420
Follow
She lost faith around week 6 of flower. My own fault but didn't damage her to much. Look forward to the cure. They've had their 2 days of darkness and all hanging on 60/60. Will look back in 5 days to see where we're at 🌱💚

Likes
6
Share


@BLAZED
Follow
Week 11 (26-12 to 1-1)
26-12
Temperature: 25.9 degrees (lights on) 19.2 degrees (lights off)
Humidity: 82% (highest) 47% (lowest)
Watering: 1000 ml. PH: 6.5 EC: 1.2
(1gr Calcium, 0.2ml Silica, 0.3ml CalMag, 1ml SugarRoyal, 1ml PowerBuds, 2ml AlgaBloom per liter)
I tested my PH pen, and it came out 0.4 too high, so i recalibrated it.
The light distance is 35/37 cm, and at 80% strength.
27-12
Temperature: 26.1 degrees (lights on) 18.1 degrees (lights off)
Humidity: 68% (highest) 48% (lowest)
Watering: None.
28-12
Temperature: 26.9 degrees (lights on) 19.2 degrees (lights off)
Humidity: 69% (highest) 49% (lowest)
Watering: None.
29-12
Temperature: 26.4 degrees (lights on) 20.1 degrees (lights off)
Humidity: 72% (highest) 50% (lowest)
Watering: 1000 ml. EC: 0.5 PH: 6.4
(1gr Calcium, 0.2ml Silica 0.3ml CalMag per liter)
30-12
Temperature: 24.6 degrees (lights on) 18.7 degrees (lights off)
Humidity: 71% (highest) 50% (lowest)
Watering: None.
31-12
Not at home.
1-1
Temperature: 25 degrees (lights on) 18 degrees (lights off)
Humidity: 68% (highest) 45% (lowest)
Watering: 1000 ml. PH: 5.8 EC: 1.8
As you can see the PH from the feeding water is lower then normal, this is because someone suggested that i can try to lower the PH as my PH pen was a bit too high, aswell as my soil PH.
Lamp is at 80% and 40 cm distance.
Happy new year growmies!


Processing
Likes
7
Share


@Cogollo_eu
Follow
**Encontrarás la traducción a español al final de la descripción**
From/Desde: 22/03/19 || To/Hasta: 28/03/19
From day/Desde día: 29 || To day/Hasta día: 35
You can find the Gorillas Diary here:
** Podéis encontrar el diario de las Gorilla aquí:**
https://growdiaries.com/diaries/25675-makingmoney-with-gorilla-mm-vs-gorilla
-----IMAGES & VIDEOS-----
Video 1:
Exactly the same video as 2 but accelerated +400% to fix it to 1 minute for instagram.
Video 2:
7 days (29~35) TimeLapse, 1 image each 60 secs @ 30 fps
Video 9:
An overview video not as awesome as the music 😂💪
Video 10:
Myself working on the babies, lowering tops, topping & training.
-----WEEK SUMMARY-----
Well, now i'm getting a bit scared as i adventured myself into Photoperiod, high training, full topping... in indoors at once. I feel that plants are going good, but i really don't know what am i doing, and if i'm doing well. Also i don't know how much time should i give them of vegetation stage, because i don't want to eternalize myself with this tent, so i'm planning to leave this upcoming 6th week and maybe the 7th of vegetation, but no more. Anyway they look pretty atm 😻.
-----WATERING CALENDAR-----
24/03/19 - 1.000 ml with all week nutrients @ 0.9 E.C. PH5.8
*****ESPAÑOL*****
-----IMÁGENES & VÍDEOS-----
Vídeo 1:
TimeLapse, exactamente el mismo vídeo que el 2 pero acelerado a un poco más del 300% para ajustarlo a 1 minuto para Instagram.
Vídeo 2:
7 días (29~35) TimeLapse, 1 imagen cada 60 segundos @ 30 fps.
Vídeo 9:
Un vídeo general no tan increíble como la música de fondo 😂💪.
Video 10:
Yo trabajando en las pequeñas, rebajando las alturas, haciendo topping y entrenando.
-----SUMARIO SEMANAL-----
Bueno, ahora estoy empezando a estar asustado. Me he aventurado a probar con fotodependientes, entrenamiento fuerte y super topping, todo a la vez. Siento que las plantas van bien, pero realmente no se lo que estoy haciendo ni si lo estoy haciendo bien. También tengo dudas sobre cuento tiempo más dejarlas en estado vegetativo ya que no me quiero eternizar con este armario. Por lo que estoy planeando dejar esta sexta semana de crecimiento y quizás una séptima, pero no más. Aun así y con todo, se ven preciosas 😻.
-----CALENDARIO DE RIEGO-----
24/03/19 - 1.000 ml con todos los nutrientes semanales @ 0.9 E.C. PH5.8

Likes
25
Share


@Ultraviolet
Follow
ANTHOCYANIN production is primarily controlled by the Cryptochrome (CR1) Photoreceptor ( !! UV and Blue Spectrums are primary drivers in the production of the pigment that replaces chlorophyll, isn't that awesome!
1. Diverse photoreceptors in plants
Many civilizations, including the sun god of ancient Egypt, thought that the blessings of sunlight were the source of life. In fact, the survival of all life, including humans, is supported by the photosynthesis of plants that capture solar energy. Plants that perform photosynthesis have no means of transportation except for some algae. Therefore, it is necessary to monitor various changes in the external environment and respond appropriately to the place to survive. Among various environmental information, light is especially important information for plants that perform photosynthesis.
In the process of evolution, plants acquired phytochrome, which mainly receives light in the red light region, and multiple blue light receptors, including his hytropin and phototropin, in order to sense the light environment. .. In addition to these, an ultraviolet light receptor named UVR8 was recently discovered. The latest image of the molecular structure and function of these various plant photoreceptors (Fig. 1), focusing on phytochrome and phototropin.
Figure 1
Ultraviolet-visible absorption spectra of phytochrome, cryptochrome, phototropin, and UVR8. The dashed line represents each bioactive absorption spectrum.
2. Phytochrome; red-far red photoreversible molecular switch
What is phytochrome?
Phytochrome is a photochromic photoreceptor, and has two absorption types, a red light absorption type Pr (absorption maximum wavelength of about 665 nm) and a far-red light absorption type Pfr (730 nm). Reversible light conversion between the two by red light and far-red light, respectively(Fig. 1A, solid line and broken line). In general, Pfr is the active form that causes a physiological response. With some exceptions, phytochrome can be said to function as a photoreversible molecular switch. The background of the discovery is as follows. There are some types of plants that require light for germination (light seed germination). From that study, it was found that germination was induced by red light, the effect was inhibited by subsequent far-red light irradiation, and this could be repeated, and the existence of photoreceptors that reversibly photoconvert was predicted. In 1959, its existence was confirmed by the absorption spectrum measurement of the yellow sprout tissue, and it was named phytochrome. Why does the plant have a sensor to distinguish between such red light and far-red light? There is no big difference between the red and far-red light regions in the open-field spectrum of sunlight, but the proportion of red light is greatly reduced due to the absorption of chloroplasts in the shade of plants. Similar changes in light quality occur in the evening sunlight. Plants perceive this difference in light quality as the ratio of Pr and Pfr, recognize the light environment, and respond to it.
Subsequent studies have revealed that it is responsible for various photomorphogenic reactions such as photoperiodic flowering induction, shade repellent, and deyellowing (greening). Furthermore, with the introduction of the model plant Arabidopsis thaliana (At) and the development of molecular biological analysis methods, research has progressed dramatically, and his five types of phytochromes (phyA-E) are present in Arabidopsis thaliana. all right. With the progress of the genome project, Fi’s tochrome-like photoreceptors were found in cyanobacteria, a photosynthetic prokaryotes other than plants. Furthermore, in non-photosynthetic bacteria, a homologue molecule called bacteriophytochrome photoreceptor (BphP) was found in Pseudomonas aeruginosa (Pa) and radiation-resistant bacteria (Deinococcus radiodurans, Dr).
Domain structure of phytochrome molecule
Phytochrome molecule can be roughly divided into N-terminal side and C-terminal side region. PAS (Per / Arndt / Sim: blue), GAF (cGMP phosphodiesterase / adenylyl cyclase / FhlA: green), PHY (phyto-chrome: purple) 3 in the N-terminal region of plant phytochrome (Fig. 2A) There are two domains and an N-terminal extension region (NTE: dark blue), and phytochromobilin (PΦB), which is one of the ring-opening tetrapyrroles, is thioether-bonded to the system stored in GAF as a chromophore. ing. PAS is a domain involved in the interaction between signal transduction-related proteins, and PHY is a phytochrome-specific domain. There are two PASs and her histidine kinase-related (HKR) domain (red) in the C-terminal region, but the histidine essential for kinase activity is not conserved.
3. Phototropin; photosynthetic efficiency optimized blue light receptor
What is phototropin?
Charles Darwin, who is famous for his theory of evolution, wrote in his book “The power of move-ment in plants” published in 1882 that plants bend toward blue light. Approximately 100 years later, the protein nph1 (nonphoto-tropic hypocotyl 1) encoded by one of the causative genes of Arabidopsis mutants causing phototropic abnormalities was identified as a blue photoreceptor. Later, another isotype npl1 was found and renamed phototropin 1 (phot1) and 2 (phot2), respectively. In addition to phototropism, phototropin is damaged by chloroplast photolocalization (chloroplasts move through the epidermal cells of the leaves and gather on the cell surface under appropriate light intensity for photosynthesis. As a photoreceptor for reactions such as escaping to the side of cells under dangerous strong light) and stomata (reactions that open stomata to optimize the uptake of carbon dioxide, which is the rate-determining process of photosynthetic reactions). It became clear that it worked. In this way, phototropin can be said to be a blue light receptor responsible for optimizing photosynthetic efficiency.
Domain structure and LOV photoreaction of phototropin molecule
Phototropin molecule has two photoreceptive domains (LOV1 and LOV2) called LOV (Light-Oxygen-Voltage sensing) on the N-terminal side, and serine / on the C-terminal side. It is a protein kinase that forms threonine kinase (STK) (Fig. 4Aa) and whose activity is regulated by light. LOV is one molecule as a chromophore, he binds FMN (flavin mononucleotide) non-covalently. The LOV forms an α/βfold, and the FMN is located on a β-sheet consisting of five antiparallel β-strands (Fig. 4B). The FMN in the ground state LOV shows the absorption spectrum of a typical oxidized flavin protein with a triplet oscillation structure and an absorption maximum wavelength of 450 nm, and is called D450 (Fig. 1C and Fig. 4E). After being excited to the singlet excited state by blue light, the FMN shifts to the triplet excited state (L660t *) due to intersystem crossing, and then the C4 (Fig. 4C) of the isoaroxazine ring of the FMN is conserved in the vicinity. It forms a transient accretionary prism with the tain (red part in Fig. 4B Eα) (S390I). When this cysteine is replaced with alanine (C / A substitution), the addition reaction does not occur. The effect of adduct formation propagates to the protein moiety, causing kinase activation (S390II). After that, the formed cysteine-flavin adduct spontaneously dissociates and returns to the original D450 (Fig. 4E, dark regression reaction).
Phototropin kinase activity control mechanism by LOV2
Why does phototropin have two LOVs? Atphot1 was found as a protein that is rapidly autophosphorylated when irradiated with blue light.
The effect of the above C / A substitution on this self-phosphorylation reaction and phototropism was investigated, and LOV2 is the main photomolecular switch in both self-phosphorylation and phototropism. It turns out that it functions as. After that, from experiments using artificial substrates, STK has a constitutive activity, LOV2 functions as an inhibitory domain of this activity, and the inhibition is eliminated by photoreaction, while LOV1 is kinase light. It was shown to modify the photosensitivity of the activation reaction. In addition to this, LOV1 was found to act as a dimerization site from the crystal structure and his SAXS. What kind of molecular mechanism does LOV2 use to photoregulate kinase activity? The following two modules play important roles in this intramolecular signal transduction.
Figure 4
(A) Domain structure of LOV photoreceptors. a: Phototropin b: Neochrome c: FKF1 family protein d: Aureochrome (B) Crystal structure of auto barley phot1 LOV2. (C) Structure of FMN isoaroxazine ring. (D) Schematic diagram of the functional domain and module of Arabidopsis thaliana phot1. L, A’α, and Jα represent linker, A’α helix, and Jα helix, respectively. (E) LOV photoreaction. (F) Molecular structure model (mesh) of the LOV2-STK sample (black line) containing A’α of phot2 obtained based on SAXS under dark (top) and under bright (bottom). The yellow, red, and green space-filled models represent the crystal structures of LOV2-Jα, protein kinase A N-lobe, and C-robe, respectively, and black represents FMN. See the text for details.
1) Jα. LOV2 C of oat phot1-to α immediately after the terminus
Rix (Jα) is present (Fig. 4D), which interacts with the β-sheet (Fig. 4B) that forms the FMN-bound scaffold of LOV2 in the dark, but unfolds and dissociates from the β-sheet with photoreaction. It was shown by NMR that it does. According to the crystal structure of LOV2-Jα, this Jα is located on the back surface of the β sheet and mainly has a hydrophobic interaction. The formation of S390II causes twisting of the isoaroxazine ring and protonation of N5 (Fig. 4C).
As a result, the glutamine side chain present on his Iβ strand (Fig. 4B) in the β-sheet rotates to form a hydrogen bond with this protonated N5. Jα interacts with this his Iβ strand, and these changes are thought to cause the unfold-ing of Jα and dissociation from the β-sheet described above. Experiments such as amino acid substitution of Iβ strands revealed that kinases exhibit constitutive activity when this interaction is eliminated, and that Jα plays an important role in photoactivation of kinases.
2) A’α / Aβ gap.
Recently, several results have been reported showing the involvement of amino acids near the A’α helix (Fig. 4D) located upstream of the N-terminal of LOV2 in kinase photoactivation. Therefore, he investigated the role of this A’α and its neighboring amino acids in kinase photoactivation, photoreaction, and Jα structural change for Atphot1. The LOV2-STK polypeptide (Fig. 4D, underlined in black) was used as a photocontrollable kinase for kinase activity analysis. As a result, it was found that the photoactivation of the kinase was abolished when amino acid substitution was introduced into the A’α / Aβ gap between A’α and Aβ of the LOV2 core. Interestingly, he had no effect on the structural changes in Jα examined on the peptide map due to the photoreaction of LOV2 or trypsin degradation. Therefore, the A’α / Aβ gap is considered to play an important role in intramolecular signal transduction after Jα.
Structural changes detected by SAXS
Structural changes of Jα have been detected by various biophysical methods other than NMR, but structural information on samples including up to STK is reported only by his results to his SAXS. Not. The SAXS measurement of the Atphot2 LOV2-STK polypeptide showed that the radius of inertia increased from 32.4 Å to 34.8 Å, and the molecular model (Fig. 4F) obtained by the ab initio modeling software GASBOR is that of LOV2 and STK. It was shown that the N lobes and C lobes lined up in tandem, and the relative position of LOV2 with respect to STK shifted by about 13 Å under light irradiation. The difference in the molecular model between the two is considered to reflect the structural changes that occur in the Jα and A’α / Aβ gaps mentioned above.
Two phototropins with different photosensitivity
In the phototropic reaction of Arabidopsis Arabidopsis, Arabidopsis responds to a very wide range of light intensities from 10–4 to 102 μmol photon / sec / m2. At that time, phot1 functions as an optical sensor in a wide range from low light to strong light, while phot2 reacts with light stronger than 1 μmol photon / sec / m2. What is the origin of these differences? As is well known, animal photoreceptors have a high photosensitivity due to the abundance of rhodopsin and the presence of biochemical amplification mechanisms. The exact abundance of phot1 and phot2 in vivo is unknown, but interesting results have been obtained in terms of amplification.
The light intensity dependence of the photoactivation of the LOV2-STK polypeptide used in the above kinase analysis was investigated.
It was found that phot1 was about 10 times more photosensitive than phot2. On the other hand, when the photochemical reactions of both were examined, it was found that the rate of the dark return reaction of phot1 was about 10 times slower than that of phot2. This result indicates that the longer the lifetime of S390II, which is in the kinase-activated state, the higher the photosensitivity of kinase activation. This correlation was further confirmed by extending the lifespan of her S390II with amino acid substitutions. This alone cannot explain the widespread differences in photosensitivity between phot1 and phot2, but it may explain some of them. Furthermore, it is necessary to investigate in detail protein modifications such as phosphorylation and the effects of phot interacting factors on photosensitivity.
Other LOV photoreceptors Among fern plants and green algae, phytochrome ɾphotosensory module (PSM) on the N-terminal side and chimera photoreceptor with full-length phototropin on the C-terminal side, neochrome (Fig. There are types with 4Ab). It has been reported that some neochromes play a role in chloroplast photolocalization as a red light receiver. It is considered that fern plants have such a chimera photoreceptor in order to survive in a habitat such as undergrowth in a jungle where only red light reaches.
In addition to this, plants have only one LOV domain, and three proteins involved in the degradation of photomorphogenesis-related proteins, FKF1 (Flavin-binding, Kelch repeat, F-box 1, ZTL (ZEITLUPE)), LKP2 ( There are LOV Kelch Protein2) (Fig. 4Ac) and aureochrome (Fig. 4Ad), which has a bZip domain on the N-terminal side of LOV and functions as a gene transcription factor.
4. Cryptochrome and UVR8
Cryptochrome is one of the blue photoreceptors and forms a superfamily with the DNA photoreceptor photolyase. It has FAD (flavin adenine dinucle-otide) as a chromophore and tetrahydrofolic acid, which is a condensing pigment. The ground state of FAD is considered to be the oxidized type, and the radical type (broken line in Fig. 1B) generated by blue light irradiation is considered to be the signaling state. The radical type also absorbs in the green to orange light region, and may widen the wavelength region of the plant morphogenesis reaction spectrum. Cryptochrome uses blue light to control physiological functions similar to phytochrome.
It was identified as a photoreceptor from one of the causative genes of UVR8 Arabidopsis thaliana, and the chromophore is absorbed in the UVB region by a Trp triad consisting of three tryptophans (Fig. 1D). It is involved in the biosynthesis of flavonoids and anthocyanins that function as UV scavengers in plants.
Conclusion
It is thought that plants have acquired various photoreceptors necessary for their survival during a long evolutionary process. The photoreceptors that cover the existing far-red light to UVB mentioned here are considered to be some of them. More and more diverse photoreceptor genes are conserved in cyanobacteria and marine plankton. By examining these, it is thought that the understanding of plant photoreceptors will be further deepened.


Likes
15
Share


Likes
10
Share


@Sadhus
Follow
Rempotage en 13 litres après quelques signes de feuilles jaunes sur certaines , plante charnue trapue a feuilles large , ormi quelque feuilles cramé sur certaines les 7 sont jolies bientôt la floraison et j'ai hâte de voir sa! 100% organic et au naturel zero stress no topping no lst
#kannabia
#madamegrow
#trolmaster

Likes
10
Share
@Yamamoto420
Follow
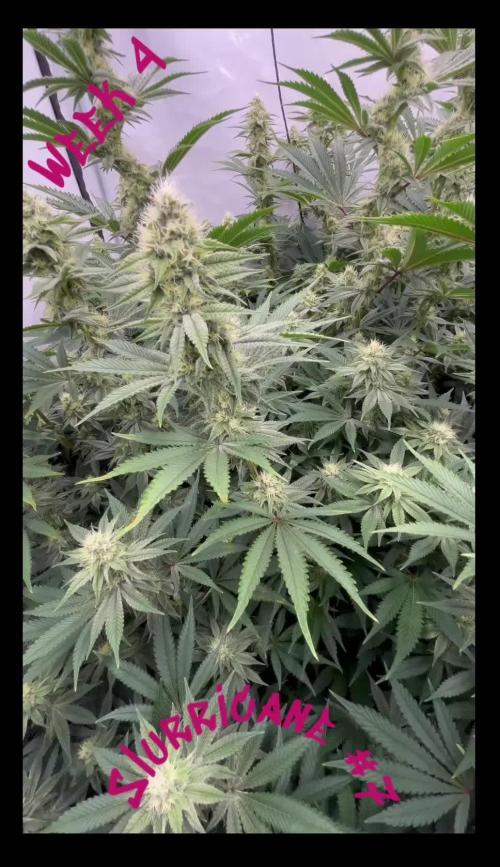
Week 4 day 22 the ladies stop stretching I had to do important deflation for the under canopy and stems where the light is not reaching, I don’t want popcorn buds. So far so good.


Likes
1
Share


@SlamFM
Follow
Feeding;
2.5ml/gal - Cal-Mag
.75g/gal - B1
.75g/gal - B2
1.5g/gal - Full Tilt
2ml/gal - Overdrive
11/1/24 - Start of Week 9
Likes
Comments
Share


@Backyardnewbie
Follow
Moved light to 3ft above plants. 400ppfd plants are reacting well.


Likes
10
Share


@Stanp
Follow
This week starts with smelly Blue Cheese Automatic. It’s growing great. Week 9
The Fruit spirit is getting bushier and looks healthy. Week 10
3G is growing slowly but surely. Looks great! Week 6th
Likes
3
Share


@OldskoolHed
Follow
In stretch mode at about 750-800 ppfd currently on full bloom nutrients. Watering about 1.75 gal every 4th day.
Likes
102
Share


@Hashy
Follow
Week 3
Light settings
18/6 on at 6.00am off 0.00am
Light power= 46% 109w
Radiator settings
LIghts on
Turn on if temp drops below 21.4c
Turn off if temp goes above 21.5c
Lights off
Turn on if temp drops below 19c
Turn off if temp goes above 19.1c
Humidifier settings
LIghts on
Turn on if humidity drops below 59.9%
Turn off if humidity goes above 60%
LIghts off
Turn on if humidity drops below 49.9%
Turn off if humidity goes above 50%
Extractor settings
temperature 24c with 1c steps
Humidity 62% with 2% steps
Max speed 8
Min speed 1
VPD aim 0.5-0.9
Wednesday 8/2/23 Day 15
5.00pm
Turn pots 90 deg
Thursday 9/2/23 Day 16
8.30pm
#3 Feed 1.5L Ec=1.06 Ph=6.4
Run 0.1L Ec=2.4 Ph=5.8
Moved
#3 to centre
#3 Height= 17CM Dist= 53CM DLI=22.6
Friday 10/2/23 Day 17
Did nothing
#3 contemplated fiming
Saturday 11/2/23 Day 18
8.00pm
#3 moved to left and fim, should have 5 sets of nodes and then the fim part.
#3 Height= 19CM Dist= 52CM DLI= 20.0
Extractor settings
temperature 25c with 1c steps
Humidity 62% with 2% steps
Max speed 8
Min speed 1
Sunday 12/2/23 Day 19
4.30pm
Leaf tuck all 3
#3 struggled to expose nodes.
8.30pm
removed humidifier and moved pots nearer centre of the tent.
A bit more leaf tucking.
Monday 13/2/23 Day 20
7.30pm
#3 Feed 2L Ec=1.04 Ph=6.5
Run 0.22L Ec=1.99 Ph=6.0
Tuesday 14/2/23 Day 21
#3 Height=24CM Dist=46CM DLI=23.5
Round up for the week.
Again it's been a fairly productive week with the grow. Didn't quite hit my VPD target but I wasn't far from it. There is enough foliage that I managed to remove the humidifier from the tent.
#3 Gorilla Cookies FF has come on great this week. Like the Tropicana Cookies she has shot up this week and has big leaves, because of this I also attempted to fim to slow her down a bit. Out of the 3 strains in the tent this one seems to have droopy leaves a good few hours before lights out, as if it's had enough for the day and gone to bed. I don't think it's got any issues but I'll keep a closer eye on this one. One more week of Veg I feel before 12/12.
Power used for week
Light
(1.96+1.96+1.96+1.96+1.96+1.95+1.95)=13.7Kw
Extractor
(0.05+0.05+0.05+0.06+0.06+0.06+0.07)=0.4Kw
Fans
(0.31+0.30+0.30+0.30+0.3+0.31+0.39)=2.21Kw
Humid
(0.05+0.02+0.0+0.0+++)=0.07Kw
Radiator
(1.44+0.9+1.04+0.68+0.6+0.92+2.61)=8.19Kw
Total for the week=24.57Kw
Back in a week.
Thanks for stopping by.
Likes
26
Share
@TrickzGrowz
Follow
Servus Moin!
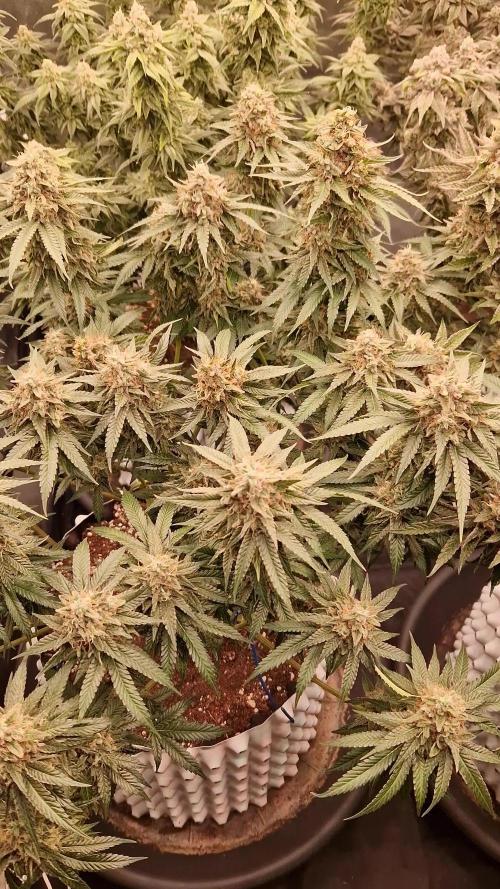
Die Buds entwickeln sich langsam richtig aus. Sie sind aber jetzt schon riesig und richtig fest.
Super klebrig und mega süß im Geruch.

Likes
10
Share


@portcityplug
Follow
I did HST on B and put one of the branches into the centre for a better spread of the light I also took off all the under foliage from A give it some better airflow
did a water change on the 26 everything is looking good to me a little burning on some leafs but light moved up now
Likes
12
Share


@Roberts
Follow
Ze Chem Bang is growing well. I did a solution change today. I switched her light times 2 weeks ago. Sorry I missed a update. She was lollipopped, and defoliated to open her up for stretching. Nothing else is really going on yet. Thank you Terpyz Mutant Genetics, and Spider Farmer. 🤜🏻🤛🏻🌱🌱🌱
Thank you grow diaries community for the 👇likes👇, follows, comments, and subscriptions on my YouTube channel👇.
❄️🌱🍻 Happy Growing 🌱🌱🌱
https://youtube.com/channel/UCAhN7yRzWLpcaRHhMIQ7X4g.
